Sulfolobus solfataricus
| Sulfolobus solfataricus | |
|---|---|
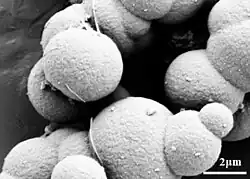 | |
| EM admission of cells of S. solfataricus fixed on a substrate | |
Scientific classification  | |
| Domain: | Archaea |
| Kingdom: | Thermoproteati |
| Phylum: | Thermoproteota |
| Class: | Thermoprotei |
| Order: | Sulfolobales |
| Family: | Sulfolobaceae |
| Genus: | Sulfolobus |
| Species: | S. solfataricus |
| Binomial name | |
| Sulfolobus solfataricus Zillig et al. 1980 | |
| Synonyms | |
| |
Saccharolobus solfataricus is a species of thermophilic archaeon. It was transferred from the genus Sulfolobus to the new genus Saccharolobus with the description of Saccharolobus caldissimus in 2018.[1] Sulfolobus solfataricus is now a basonym for Saccharolobus solfataricus.
It was discovered and isolated from the Solfatara volcano (Pisciarelli-Campania, Italy) in 1980 by two German microbiologists, Karl Setter and Wolfram Zillig.[2] These organisms are not isolated in volcanoes, however; they are found all over the world, in places such as hot springs.
The species grows best in temperatures around 80 °C (176 °F), a pH level between 2 and 4, and with enough sulfur for S. solfataricus to metabolize to gain energy. These conditions qualify it as an extremophile, and it is known as a thermoacidophile because of its preference for high temperatures and low pH levels. It is aerobic and heterotropic, due to its metabolic system.[3] As an autotroph, it receives energy by growing on sulfur or a variety of organic compounds.[4] It usually has a spherical shape, with several lobes.
It is the most widely-studied organism in the Thermoproteota branch. S. solfataricus are examined for their methods of DNA replication, cell cycle, chromosomal integration, transcription, RNA processing, and translation. Data indicates that the organism has a large percentage of archaeal-specific genes, which can be utilized to show differences between the three domains of life: Archaea, bacteria and eukaryote.
Genome
S. solfataricus is the most studied microorganism from molecular, genetic, and biochemical points of view for its ability to thrive in extreme environments. It can grow easily in the laboratory and can exchange genetic material through transformation, transduction, and conjugation.
The main reason for sequencing these microorganisms is to study the thermostability of proteins which normally denature at a high temperature. The complete genome sequence of S. solfataricus was completed in 2001.[5] There are 2,992,245 base pairs on a single chromosome, which encode 2,977 proteins and a large amount of RNA. One-third of S. solfataricus' encoded proteins have no homologs in other genomes. For the remaining encoded proteins, 40 percent are specific to Archaea, 12 percent are shared with bacteria, and 2.3 percent are shared with eukaryotes;[6] 33 percent of these proteins are encoded exclusively in Sulfolobus. Many open reading frames (ORFs) are very similar in Thermoplasma.[3]
Small nucleolar RNAs (snoRNAs), already present in eukaryotes, have also been identified in S. solfataricus and S. acidolcaldarius; they are known for their roles in post-transcriptional modifications and removal of introns from ribosomal RNA in eukaryotes.[7]
The genome of S. solfataricus is characterized by short tandem repeats, insertion, and repetitive elements. It is diverse, with 200 different insertion-sequence elements.
Thermophilic reverse gyrase
Stabilization of DNA structure against denaturation in Archaea is due to reverse gyrase, a thermophilic enzyme in hyper-thermophilic and thermophilic Archaea and bacteria. Two genes in Sulfolobus encode a reverse gyrase.[8] It is defined as an atypical DNA topoisomerase, and the basic activity is the production of positive supercoils in a closed circular DNA. Positive supercoiling is important to prevent the formation of open complexes. Reverse gyrases are composed of two domains; the first is the helicase, and the second is the topoisomerase I. A possible role of reverse gyrase is the use of positive supercoiling to assemble chromatin-like structures.[9] In 1997, scientists discovered another important feature of Sulfolobus: a type II topoisomerase (TopoVI) whose A subunit is homologous to the meiotic recombination factor Spo11, which plays an importaant role in initiating meiotic recombination in eukaryotes.[10][11] S. solfataricus is composed of three topoisomerases (TopA and two reverse gyrases, TopR1 and TopR2), and TopoVI.[12]
DNA binding proteins
In the phylum Thermoproteota, three proteins which bind to the minor groove of DNA-like histones (Alba, Cren7, and Sso7d) are modified after the translation process. These histones are small and have been found in several strains of Sulfolobus, but not in other genomes. Chromatin proteins in Sulfolobus are one to five percent of the total genome; they can have structural and regulatory functions, and look like human HMG-box proteins because of their influence on genomes, expression, stability, and epigenetic processes.[13] In species lacking histones, they can be acetylated and methylated like eukaryotic histones.[14][15][16][17] Sulfolobus strains have different, peculiar DNA binding proteins such as the Sso7d protein family. They stabilize the DNA's structure, preventing denaturation at high temperatures and promoting annealing above the melting point.[18]
The main component of Archaea chromatin is the Sac10b-family protein known as Alba (an acronym for "acetylation lowers binding affinity").[19][20] These proteins are small, basic, and dimeric nucleic acid-binding proteins which are conserved in most sequenced Archaea genomes.[21][22] The acetylation of Alba affects promoter access and transcription in vitro; the methylation state of another Sulfolobus chromatin protein, Sso7D, is altered by culture temperature.[23][24]
The work of Wolfram Zillig's group, which presented early evidence of the eukaryotic characteristics of transcription in Archaea, has made Sulfolobus an ideal model system for transcription studies. Studies in Sulfolobus and other Archaea species focus on the composition, function, and regulation of the transcription machinery and on fundamental conserved aspects of this process in eukaryotes and Archaea.[25]
DNA transfer
Exposure of Saccharolobus solfataricus to DNA-damaging agents, such as ultraviolet (UV) irradiation, bleomycin, or mitomycin C, induces cellular aggregation (gathering).[26] Other physical stressors, such as changes in pH or temperature, do not induce aggregation; this suggests that it is caused specifically by DNA damage. Ajon et al.[27] showed that UV-induced cellular aggregation often mediates chromosomal-marker exchange. Recombination rates exceeded those of uninduced cultures by up to three orders of magnitude. Frols et al.[26][28] and Ajon et al.[27] hypothesized that UV-induced DNA transfer and subsequent homologous recombinational repair is an important mechanism to maintain chromosome integrity. This response may be a primitive form of sexual interaction, similar to the better-studied bacterial transformation also associated with DNA transfer between cells and leading to homologous recombinational repair of DNA damage.[29]
Metabolism
Sulfolobus solfataricus is known to grow by chemoorganotrophy in the presence of oxygen on a variety of organic compounds, such as sugars, alcohols, amino acids, and aromatic compounds like phenol.[30] It uses a modified Entner-Doudroff pathway for glucose oxidation, and the resulting pyruvate molecules can be mineralized in a citric acid cycle.[30]
Molecular oxygen is the only known electron acceptor at the end of the electron transport chain.[31] Other than organic molecules, this Archaea species can also use hydrogen sulfide[6] and sulfur as electron donors and fix CO2, possibly by means of the HP/HB cycle,[30] making it also capable of living by chemoautotrophy. Recent studies have also found the ability to grow, albeit slowly, by oxidizing molecular hydrogen.[1]
Ferredoxin
Ferredoxin is thought to be the major metabolic electron carrier in S. solfataricus. This contrasts with most bacterial and eukaryote species, which generally rely on nicotinamide adenine dinucleotide hydrogen (NADH) as the main electron carrier. S. solfataricus has strong eukaryotic features coupled with uniquely archaeal-specific abilities. The findings arose from the methods of their DNA mechanisms, cell cycles, and transitional apparatus, and was a prime example of the differences found in Thermoproteota and "Euryarchaeota".[6][32]
Ecology
Habitat

S. solfataricus is an extreme thermophile in the Archaea domain. Strong volcanic-activity areas with high temperatures and very acidic pH provide the best growth conditions for S. solfataricus and members of the related genus, Sulfolobus.[33] These conditions are typical of volcanic areas, such as geysers or thermal springs. The most-studied countries where these microorganisms are found are the U.S. (Yellowstone National Park),[34] New Zealand,[35] Iceland and Italy, all known for volcanic phenomena. A study conducted by a team of Indonesian scientists has also indicated a Sulfolobus community in West Java, confirming that high temperatures, low pH, and the presence of sulfur are necessary conditions for the growth of these microbes.[36]
Soil acidification
S. solfataricus can oxidize sulfur according to metabolic strategy. One product of these reactions is H+, and it will slowly acidify the surrounding area. Soil acidification increases in places where there are emissions of pollutants from industrial activity. This process reduces the number of heterotrophic bacteria involved in decomposition, which is fundamental for recycling organic matter. This ultimately slows the fertilization of soil.[37]
Biotechnology
There is interest in using S. sulfataricus as a source of thermal-stability enzymes for research and diagnostics, as well as industries such as food, textiles, cleaning, and pulp and paper. This enzyme is overloaded due to its catalytic diversity, high pH, temperature stability, increased resistance to organic solvents, and resistance to proteolysis.[38][39] Tetraether lipids, membrane vesicles with antimicrobial properties, trehalose components, and β-galactooligosaccharides are becoming increasingly important.[40]
β-galactosidase
The thermostable enzyme β-Galactosidase was isolated from the extreme thermophile archaebacterial S. solfataricus strain MT-4. This enzyme is used in many industrial processes of lactose-containing fluids by purifying and stabilizing their physiochemical properties.[41]
Proteases
Industry is interested in stable proteases, and a number of Sulfolobus proteases have been studied.[42] An active aminopeptidase associated with the chaperonin of S. solfataricus MT4 was described.[43] Sommaruga et al. improved the stability and reaction yield of a carboxypeptidase from S. solfataricus MT4 with magnetic nanoparticles in 2014, immobilizing the enzyme.[44]
Esterases and lipases
A thermostable extracellular lipolytic enzyme serine, arylesterase, was noted for its hydrolysis of organophosphates from the thermoacidophilic archaeon S. solfataricus P1.[45]
Chaperonins
In reaction to temperature shock (50.4 °C) in E. coli cells, a tiny warm stun protein (S.so-HSP20) from S.solfataricus P2 has been used to improve tolerance to temperature.[46] Since chaperonin Ssocpn (920 kDa), which includes adenosine triphosphate (ATP), K+, and Mg2 +, has not produced additional proteins in S. solfataricus to supply collapsed and dynamic proteins from denatured materials. It was stored on an ultrafiltration cell while the renatured substrates were moving through the film.[47]
Liposomes
Because of its tetraether lipid material, the membrane of extreme thermophilic Archaea is unique in composition. Archaea lipids are a promising source of liposomes with stable temperature and pH and tightness against the leakage of solute, and are possible instruments for the delivery of medicines, vaccines, and genes.[48]
See also
References
- 1 2 Sakai HD, Kurosawa N (April 2018). "Saccharolobus caldissimus gen. nov., sp. nov., a facultatively anaerobic iron-reducing hyperthermophilic archaeon isolated from an acidic terrestrial hot spring, and reclassification of Sulfolobus solfataricus as Saccharolobus solfataricus comb. nov. and Sulfolobus shibatae as Saccharolobus shibatae comb. nov". International Journal of Systematic and Evolutionary Microbiology. 68 (4): 1271–1278. doi:10.1099/ijsem.0.002665. PMID 29485400. S2CID 4528286.
- ↑ "Where was Sulfolobus solfataricus first found?". www.intercept.cnrs.fr. 15 January 2019.
- 1 2 Ciaramella M, Pisani FM, Rossi M (August 2002). "Molecular biology of extremophiles: recent progress on the hyperthermophilic archaeon Sulfolobus". Antonie van Leeuwenhoek. 81 (1–4): 85–97. doi:10.1023/A:1020577510469. PMID 12448708. S2CID 8330296.
- ↑ Brock TD, Brock KM, Belly RT, Weiss RL (1972). "Sulfolobus: a new genus of sulfur-oxidizing bacteria living at low pH and high temperature". Archiv für Mikrobiologie. 84 (1): 54–68. Bibcode:1972ArMic..84...54B. doi:10.1007/bf00408082. PMID 4559703. S2CID 9204044.
- ↑ Charlebois RL, Gaasterland T, Ragan MA, Doolittle WF, Sensen CW (June 1996). "The Sulfolobus solfataricus P2 genome project". FEBS Letters. 389 (1): 88–91. Bibcode:1996FEBSL.398R.343.. doi:10.1016/s0014-5793(97)81281-1. PMID 8682213. S2CID 221414122.
- 1 2 3 She Q, Singh RK, Confalonieri F, Zivanovic Y, Allard G, Awayez MJ, et al. (July 2001). "The complete genome of the crenarchaeon Sulfolobus solfataricus P2". Proceedings of the National Academy of Sciences of the United States of America. 98 (14): 7835–40. Bibcode:2001PNAS...98.7835S. doi:10.1073/pnas.141222098. PMC 35428. PMID 11427726.
- ↑ Omer AD, Lowe TM, Russell AG, Ebhardt H, Eddy SR, Dennis PP (April 2000). "Homologs of small nucleolar RNAs in Archaea". Science. 288 (5465): 517–22. Bibcode:2000Sci...288..517O. doi:10.1126/science.288.5465.517. PMID 10775111. S2CID 15552500.
- ↑ Couturier M, Bizard AH, Garnier F, Nadal M (September 2014). "Insight into the cellular involvement of the two reverse gyrases from the hyperthermophilic archaeon Sulfolobus solfataricus". BMC Molecular Biology. 15 (1) 18. doi:10.1186/1471-2199-15-18. PMC 4183072. PMID 25200003.
- ↑ Déclais AC, Marsault J, Confalonieri F, de La Tour CB, Duguet M (June 2000). "Reverse gyrase, the two domains intimately cooperate to promote positive supercoiling". The Journal of Biological Chemistry. 275 (26): 19498–504. doi:10.1074/jbc.m910091199. PMID 10748189.
- ↑ Bergerat A, de Massy B, Gadelle D, Varoutas PC, Nicolas A, Forterre P (March 1997). "An atypical topoisomerase II from Archaea with implications for meiotic recombination". Nature. 386 (6623): 414–7. Bibcode:1997Natur.386..414B. doi:10.1038/386414a0. PMID 9121560. S2CID 4327493.
- ↑ Forterre P, Bergerat A, Lopez-Garcia P (May 1996). "The unique DNA topology and DNA topoisomerases of hyperthermophilic archaea". FEMS Microbiology Reviews. 18 (2–3): 237–48. doi:10.1111/j.1574-6976.1996.tb00240.x. PMID 8639331.
- ↑ Couturier M, Gadelle D, Forterre P, Nadal M, Garnier F (November 2019). "The reverse gyrase TopR1 is responsible for the homeostatic control of DNA supercoiling in the hyperthermophilic archaeon Sulfolobus solfataricus". Molecular Microbiology. 113 (2): 356–368. doi:10.1111/mmi.14424. PMID 31713907. S2CID 207945754.
- ↑ Malarkey CS, Churchill ME (December 2012). "The high mobility group box: the ultimate utility player of a cell". Trends in Biochemical Sciences. 37 (12): 553–62. doi:10.1016/j.tibs.2012.09.003. PMC 4437563. PMID 23153957.
- ↑ Payne S, McCarthy S, Johnson T, North E, Blum P (November 2018). "Sulfolobus solfataricus". Proceedings of the National Academy of Sciences of the United States of America. 115 (48): 12271–12276. doi:10.1073/pnas.1808221115. PMC 6275508. PMID 30425171.
- ↑ Guagliardi A, Cerchia L, Moracci M, Rossi M (October 2000). "The chromosomal protein sso7d of the crenarchaeon Sulfolobus solfataricus rescues aggregated proteins in an ATP hydrolysis-dependent manner". The Journal of Biological Chemistry. 275 (41): 31813–8. doi:10.1074/jbc.m002122200. PMID 10908560.
- ↑ Shehi E, Granata V, Del Vecchio P, Barone G, Fusi P, Tortora P, Graziano G (July 2003). "Thermal stability and DNA binding activity of a variant form of the Sso7d protein from the archeon Sulfolobus solfataricus truncated at leucine 54". Biochemistry. 42 (27): 8362–8. doi:10.1021/bi034520t. PMID 12846585.
- ↑ Baumann H, Knapp S, Karshikoff A, Ladenstein R, Härd T (April 1995). "DNA-binding surface of the Sso7d protein from Sulfolobus solfataricus". Journal of Molecular Biology. 247 (5): 840–6. doi:10.1006/jmbi.1995.0184. PMID 7723036.
- ↑ Guagliardi A, Napoli A, Rossi M, Ciaramella M (April 1997). "Annealing of complementary DNA strands above the melting point of the duplex promoted by an archaeal protein". Journal of Molecular Biology. 267 (4): 841–8. doi:10.1006/jmbi.1996.0873. PMID 9135116.
- ↑ Forterre P, Confalonieri F, Knapp S (May 1999). "Identification of the gene encoding archeal-specific DNA-binding proteins of the Sac10b family". Molecular Microbiology. 32 (3): 669–70. doi:10.1046/j.1365-2958.1999.01366.x. PMID 10320587. S2CID 28146814.
- ↑ Xue H, Guo R, Wen Y, Liu D, Huang L (July 2000). "An abundant DNA binding protein from the hyperthermophilic archaeon Sulfolobus shibatae affects DNA supercoiling in a temperature-dependent fashion". Journal of Bacteriology. 182 (14): 3929–33. doi:10.1128/JB.182.14.3929-3933.2000. PMC 94576. PMID 10869069.
- ↑ Goyal M, Banerjee C, Nag S, Bandyopadhyay U (May 2016). "The Alba protein family: Structure and function". Biochimica et Biophysica Acta (BBA) - Proteins and Proteomics. 1864 (5): 570–83. doi:10.1016/j.bbapap.2016.02.015. PMID 26900088.
- ↑ Wardleworth BN, Russell RJ, Bell SD, Taylor GL, White MF (September 2002). "Structure of Alba: an archaeal chromatin protein modulated by acetylation". The EMBO Journal. 21 (17): 4654–62. doi:10.1093/emboj/cdf465. PMC 125410. PMID 12198167.
- ↑ Bell SD, Botting CH, Wardleworth BN, Jackson SP, White MF (April 2002). "The interaction of Alba, a conserved archaeal chromatin protein, with Sir2 and its regulation by acetylation". Science. 296 (5565): 148–51. Bibcode:2002Sci...296..148B. doi:10.1126/science.1070506. PMID 11935028. S2CID 27858056.
- ↑ Baumann H, Knapp S, Lundbäck T, Ladenstein R, Härd T (November 1994). "Solution structure and DNA-binding properties of a thermostable protein from the archaeon Sulfolobus solfataricus". Nature Structural Biology. 1 (11): 808–19. doi:10.1038/nsb1194-808. PMID 7634092. S2CID 37220619.
- ↑ Zillig W, Stetter KO, Janeković D (June 1979). "DNA-dependent RNA polymerase from the archaebacterium Sulfolobus acidocaldarius". European Journal of Biochemistry. 96 (3): 597–604. doi:10.1111/j.1432-1033.1979.tb13074.x. PMID 380989.
- 1 2 Fröls S, Ajon M, Wagner M, Teichmann D, Zolghadr B, Folea M, et al. (November 2008). "UV-inducible cellular aggregation of the hyperthermophilic archaeon Sulfolobus solfataricus is mediated by pili formation" (PDF). Molecular Microbiology. 70 (4): 938–52. doi:10.1111/j.1365-2958.2008.06459.x. PMID 18990182.
- 1 2 Ajon M, Fröls S, van Wolferen M, Stoecker K, Teichmann D, Driessen AJ, et al. (November 2011). "UV-inducible DNA exchange in hyperthermophilic archaea mediated by type IV pili" (PDF). Molecular Microbiology. 82 (4): 807–17. doi:10.1111/j.1365-2958.2011.07861.x. PMID 21999488.
- ↑ Fröls S, White MF, Schleper C (February 2009). "Reactions to UV damage in the model archaeon Sulfolobus solfataricus". Biochemical Society Transactions. 37 (Pt 1): 36–41. doi:10.1042/BST0370036. PMID 19143598. S2CID 837167.
- ↑ Bernstein H, Bernstein C (2010). "Evolutionary origin of recombination during meiosis". BioScience. 60 (7): 498–505. doi:10.1525/bio.2010.60.7.5. S2CID 86663600
- 1 2 3 Ulas T, Riemer SA, Zaparty M, Siebers B, Schomburg D (2012-08-31). "Genome-scale reconstruction and analysis of the metabolic network in the hyperthermophilic archaeon Sulfolobus solfataricus". PLOS ONE. 7 (8) e43401. Bibcode:2012PLoSO...743401U. doi:10.1371/journal.pone.0043401. PMC 3432047. PMID 22952675.
- ↑ Simon G, Walther J, Zabeti N, Combet-Blanc Y, Auria R, van der Oost J, Casalot L (October 2009). "Effect of O2 concentrations on Sulfolobus solfataricus P2". FEMS Microbiology Letters. 299 (2): 255–60. doi:10.1111/j.1574-6968.2009.01759.x. PMID 19735462.
- ↑ Zillig W, Stetter KO, Wunderl S, Schulz W, Priess H, Scholz I (April 1980). "The Sulfolobus-"Caldariella" group: taxonomy on the basis of the structure of DNA-dependent RNA polymerases". Archives of Microbiology. 125 (3): 259–69. Bibcode:1980ArMic.125..259Z. doi:10.1007/BF00446886. S2CID 5805400.
- ↑ Grogan DW (December 1989). "Phenotypic characterization of the archaebacterial genus Sulfolobus: comparison of five wild-type strains". Journal of Bacteriology. 171 (12): 6710–9. Bibcode:1989JBact.171.6710G. doi:10.1128/jb.171.12.6710-6719.1989. PMC 210567. PMID 2512283.
- ↑ "Sulfolobus". Microbewiki.
- ↑ Hetzer A, Morgan HW, McDonald IR, Daughney CJ (July 2007). "Microbial life in Champagne Pool, a geothermal spring in Waiotapu, New Zealand". Extremophiles. 11 (4): 605–14. Bibcode:2007Extmo..11..605H. doi:10.1007/s00792-007-0073-2. PMID 17426919. S2CID 24239907.
- ↑ Aditiawati P, Yohandini H, Madayanti F (2009). "Microbial diversity of acidic hot spring (kawah hujan B) in geothermal field of kamojang area, west java-indonesia". The Open Microbiology Journal. 3: 58–66. doi:10.2174/1874285800903010058. PMC 2681175. PMID 19440252.
- ↑ Bryant RD, Gordy EA, Laishley EJ (1979). "Effect of soil acidification on the soil microflora". Water, Air, and Soil Pollution. 11 (4): 437. Bibcode:1979WASP...11..437B. doi:10.1007/BF00283435. S2CID 96729369.
- ↑ Stepankova, Veronika (October 14, 2013). "Strategies for Stabilization of Enzymes in Organic Solvents". ACS Catalysis. 3 (12): 2823–2836. Bibcode:2013ACSCa...3.2823S. doi:10.1021/cs400684x.
- ↑ DANIEL, R. M. (1982). "A correlation between protein thermostability and resistance to proteolysis". Biochemical Journal. 207 (3): 641–644. doi:10.1042/bj2070641. PMC 1153914. PMID 6819862.
- ↑ Quehenberger, Julian (2017). "Sulfolobus – A Potential Key Organism in Future Biotechnology". Frontiers in Microbiology. 8 2474. doi:10.3389/fmicb.2017.02474. PMC 5733018. PMID 29312184.
- ↑ M. PISANI, Francesca (1990). "Thermostable P-galactosidase from the archaebacterium Sulfolobus solfataricus". European Journal of Biochemistry. 187 (2): 321–328. doi:10.1111/j.1432-1033.1990.tb15308.x. PMID 2105216.
- ↑ Hanner, Markus (1990). "Isolation and characterization of an intracellular aminopeptidase from the extreme thermophilic archaebacterium Sulfolobus solfataricus". Biochimica et Biophysica Acta (BBA) - General Subjects. 1033 (2). Elsevier B.V.: 148–153. doi:10.1016/0304-4165(90)90005-H. ISBN 0-11-753612-1. PMID 2106344.
{{cite journal}}: CS1 maint: periodical has ISBN (link) - ↑ Condo, Ivano; Ruggero, Davide (1998). "A novel aminopeptidase associated with the 60 kDa chaperonin in the thermophilic archaeon Sulfolobus solfataricus. Mol. Microbiol". Molecular Microbiology. 29 (3): 775–785. doi:10.1046/j.1365-2958.1998.00971.x. PMID 9723917.
- ↑ Sommaruga, Silvia (2014). "Immobilization of carboxypeptidase from Sulfolobus solfataricus on magnetic nanoparticles improves enzyme stability and functionality in organic media. BMC Biotechnol". BMC Biotechnology. 14 (1): 82. doi:10.1186/1472-6750-14-82. PMC 4177664. PMID 25193105.
- ↑ Park, Young-Jun (2016). "Purification and characterization of a new inducible thermostable extracellular lipolytic enzyme from the thermoacidophilic archaeon Sulfolobus solfataricus P1". Journal of Molecular Catalysis B: Enzymatic. 124: 11–19. doi:10.1016/j.molcatb.2015.11.023.
- ↑ Li, Dong-Chol (August 2011). "Thermotolerance and molecular chaperone function of the small heat shock protein HSP20 from hyperthermophilic archaeon, Sulfolobus solfataricus P2. Cell Stress Chaperones". Cell Stress & Chaperones. 17 (1): 103–108. doi:10.1007/s12192-011-0289-z. PMC 3227843. PMID 21853411.
- ↑ Cerchia, Laura (7 August 1999). "An archaeal chaperonin-based reactor for renaturation of denatured proteins. Extremophile". Extremophiles: Life Under Extreme Conditions. 4 (1): 1–7. doi:10.1007/s007920050001. PMID 10741831. S2CID 25407893.
- ↑ B. Patel, Girishchandra (1999). "Archaeobacterial Ether Lipid Liposomes (Archaeosomes) as Novel Vaccine and Drug Delivery Systems". Critical Reviews in Biotechnology. 19 (4): 317–357. doi:10.1080/0738-859991229170. PMID 10723627.
Further reading
- Fiorentino G, Del Giudice I, Petraccone L, Bartolucci S, Del Vecchio P (June 2014). "Conformational stability and ligand binding properties of BldR, a member of the MarR family, from Sulfolobus solfataricus". Biochimica et Biophysica Acta (BBA) - Proteins and Proteomics. 1844 (6): 1167–72. doi:10.1016/j.bbapap.2014.03.011. PMID 24704039.
- de Rosa M, Bemporad F, Pellegrino S, Chiti F, Bolognesi M, Ricagno S (September 2014). "Edge strand engineering prevents native-like aggregation in Sulfolobus solfataricus acylphosphatase". The FEBS Journal. 281 (18): 4072–84. doi:10.1111/febs.12861. PMID 24893801.
- Gamsjaeger R, Kariawasam R, Touma C, Kwan AH, White MF, Cubeddu L (October 2014). "Backbone and side-chain 1H, 13C and 15N resonance assignments of the OB domain of the single stranded DNA binding protein from Sulfolobus solfataricus and chemical shift mapping of the DNA-binding interface". Biomolecular NMR Assignments. 8 (2): 243–6. doi:10.1007/s12104-013-9492-4. PMID 23749431. S2CID 6388231.
- Wang J, Zhu J, Min C, Wu S (May 2014). "CBD binding domain fused γ-lactamase from Sulfolobus solfataricus is an efficient catalyst for (-) γ-lactam production". BMC Biotechnology. 14 40. doi:10.1186/1472-6750-14-40. PMC 4041915. PMID 24884655.