Haplogroup K2b (Y-DNA)
| Haplogroup K2b (P331) | |
|---|---|
 | |
| Possible time of origin | 51,800 years BP[1] |
| Coalescence age | 48,900 years BP |
| Possible place of origin | Probably South Asia, Southeast Asia,[2][3] East Asia[4] or Central Asia |
| Ancestor | K2 |
| Descendants | |
| Defining mutations | P331, CTS2019/M1205, PF5990/L405, PF5969,[5][2] |
Haplogroup K2b (P331), also known as MPS[5] is a human Y-chromosome DNA haplogroup. According to the age estimates of Tatiana Karafet et al. (2014), haplogroup K2b is around 50,000 years old, less than 3,000 years younger than K.[2]
Origins
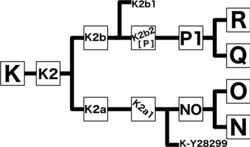
Haplogroup K2b is a primary subclade of haplogroup K2. Due to its unusually wide and rapid geographical dispersal, with at least five primary subclades (including K2b) and its basal form (K2*),[6] haplogroup K2 probably emerged in close proximity to K* and K2b. According to the population geneticist Tatiana Karafet et al. (2014), the estimated dates for the branching of K, K2, K2b and P point to a "rapid diversification" within K2 "that likely occurred in Southeast Asia," with subsequent "westward expansions" of P1, Q and R.[2]
Haplogroup K2b is a secondary subclade of haplogroup K-M9. Geneticist Spencer Wells had argued that because haplogroup K-M9 has a geographically wide distribution, the lineage may have originated near the central part of this range in the Middle East or Central Asia, perhaps in Iran or Pakistan.[7]
Basal paragroup K2b* has not been identified among living males, but was detected in the Tianyuan man found in China, an individual dated to the Upper Paleolithic (about 40,000 years BP).[8]
K2b1 (P397/P399), known previously as haplogroup MS, and haplogroup P (P-P295), also known as K2b2, are the only primary subclades of K2b. Karafet and other researchers (2014) point out that K2b1, its subclades and P* are virtually restricted geographically to South East Asia and Oceania.[2] Whereas, in a striking contrast, subclades of P1, namely Q and R, now make up "the most frequent haplogroup in Europe, the Americas, and Central Asia and South Asia".
Phylogenetic structure
- K2b (P331), also known as MPS.
- K2b1 (P397, P399), similar to the previous haplogroup MS.
- K2b1a (P405)
- K2b1a1 (P60)
- K2b1a2 (P79)
- K2b1a3 (P315)
- Haplogroup S (B254), previously known as K2b1a.
- Haplogroup M (P256), also known as K2b1b.
- K2b1a (P405)
- Haplogroup P (P-F5850)
- K2b1 (P397, P399), similar to the previous haplogroup MS.
Distribution
There is a distinct contrast between the distribution of two, de facto geographical groups comprising, respectively:
- K2*, K2b1 (all subclades), P* (also known as K2b2*; P-P295*) and P2 (also known as K2b2b; P-B253), and;
- P1 (also known as K2b2a) and its descendants, including Q and R.
To the extent that both groups overlap, it is in populations native to the southwest Pacific region, where some Negrito populations carry very high levels of K2b at the subclade level. It is carried, for instance, by more than 83% of males among the Aeta (or Agta) people of the Philippines, in the form of subclades of K2b1 (haplogroups M and S, at levels of more than 60%), as well as P*, P1*, and P2*.
Modern populations with living members of K2*, K2b1 (haplogroups M and S), P* (P-P295*) and P2 (also known as K2b2b) are the predominant haplogroups in New Guinea, some subgroups of indigenous Australians, as well as males native to other parts of Oceania and parts of Island South East Asia.
P1 (also known as K2b2a), including primary subclades such as P1c (P-M45*; previously P1), in modern times, is distributed among populations native to a wide area that includes Europe, Central Asia, South East Asia, and Native Americans.
K2b1
K2b1 is found in 83% of males of Papua New Guinea, and up to 60% in the Aeta people of the Philippines.[2] It is also found among other Melanesian populations, as well as indigenous Australians, and at lower levels amongst Polynesians.[2] It is also found in the Melanesian populations of Indonesia.
Major studies of indigenous Australian Y-DNA, published in 2014 and 2015, suggest that about 29% of indigenous Australian males belong to subclades of K2b1. That is, up to 27% indigenous Australian males carry haplogroup S1a1a1 (S-P308; previously known as K2b1a1 or K-P308),[2] and one study found that approximately 2.0% – i.e. 0.9% (11 individuals) of the sample in a study in which 45% of the total was deemed to be non-indigenous – belonged to haplogroup M1 (M-M4; also known as M-M186 and known previously as haplogroup K2b1d1). All of these males carrying M1 were Torres Strait Islanders.[9] The other Y-chromosome DNA haplogroups found were: basal K2* (K-M526), C1b2b (C-M347; previously Haplogroup C4), and basal C* (C-M130).
| Population | K2b1 (including haplogroups M & S) |
|---|---|
| Papua New Guinea | 82.76% |
| Maori | 3.82% (1.95% of those sampled, i.e. 49% of Maori males were deemed to have non-indigenous haplogroups) |
| Fiji | 60.75% |
| Solomon Islands | 71.9% |
| French Polynesia | 8% |
| Vanuatu | 76.5% |
| New Caledonia | |
| Guam | 33.3% (Small sample size) |
| Samoa | 8.04% |
| Kiribati | 0% (Small sample size) |
| Tonga | 20.69% |
| Micronesia FDR | 66.67% |
| Marshall Islands | 63.64% |
| American Samoa | |
| Northern Mariana Islands | |
| Palau | 61.5% (Small sample size) |
| Cook Islands | 3.9% |
| Wallis and Futuna | 26% |
| Tuvalu | 36% |
| Nauru | 28.6% (Small sample size) |
| Norfolk Island | |
| Niue | 0% (Small sample size) |
| Tokelau | 50% (Small sample size) |
| Hawaii | 20% (Small sample size, from FTDNA) |
| Aboriginal Australians | 29%[9] |
| Timor | 25% |
| Aeta | 60% |
| Malaysia | 2.40% (Small sample size) |
| Flores | 35% |
| Sulawesi | 11.3% |
| Sulawesi | 0% |
| East Indonesia (Lesser Sunda Islands) | 25.9% |
| Java Indonesia | 0% |
| Bali Indonesia | 0.9% |
| Sumatra Indonesia | 0% |
| Borneo Indonesia | 5.8% |
| West Papua (Papua Province, Indonesia) | 52.6% |
| West Papua (Papua Province, Indonesia) | 82.6% |
| Sumba Indonesia | 25.2% |
| Chukkese people Micronesia | 76.5% |
| Pohnpeian people Micronesia | 70% (Small sample size) |
P (K2b2)
Apart from the basal paragroup P* (K2b2), it has only one subclade: P1 (M45), also known as K2b2a – which is also the parent of the major haplogroups Q (K2b2a1) and R (K2b2a2).[2]
P (K2b2) descendant haplogroups Q (K2b2a1) and R (K2b2a2) is widely distributed among males of Native American, Central Asian, South Asian and Siberian ancestry.
Basal P* (K2b2*)
P-P295* (sometimes known as "pre-P", before P-M45 was redesignated P1) is found among 28% of males among the Aeta, as well as in Timor at 10.8%, and one case may have been found in Papua New Guinea (Kaysar et al. 2006) although this has not been verified.[2]
| Population | Rate of P* (%) | Notes |
|---|---|---|
| Papua New Guinea | 0.69 | Assumed from Kayser et al. (2006), i.e. one P* found |
| New Zealand | 0 | |
| Fiji | 0 | |
| Solomon Islands | 0 | |
| French Polynesia | 0 | |
| Vanuatu | 0 | |
| New Caledonia | ||
| Guam | 0 | |
| Samoa | 0 | |
| Kiribati | ||
| Tonga | 0 | |
| Federated States of Micronesia | 0 | |
| Marshall Islands | 0 | |
| American Samoa | ||
| Northern Mariana Islands | ||
| Palau | ||
| Cook Islands | 0 | |
| Wallis and Futuna | 0 | |
| Tuvalu | 0 | |
| Nauru | ||
| Norfolk Island | ||
| Niue | 0 | Small sample size |
| Tokelau | 0 | Small sample size |
| Hawaii | 0 | Small sample size, from FTDNA |
| Australia | 0 | |
| Timor | 10.8 | |
| Aeta | 28 | |
| Filipino Austronesian | 0 | |
| Malay | 0 | |
| Flores | 0 | |
| Sulawesi | 0.6 | |
| East Indonesia | 0 | |
| Java Indonesia | 0 | |
| Bali Indonesia | 0 | |
| Sumatra Indonesia | 0 | |
| Borneo Indonesia | 0 | |
| West Papua Province | 0 | |
| Papua Province | 0 | |
| Sumba Indonesia | 3.2 |
P1 (K2b2a)
P1 (M45/PF5962), also known as K2b2a, is hundreds of times more common than P* (K2b2; PxM45), as it includes haplogroups Q and R, is estimated as being 14,300 years younger than K2b.[2]
Many ethnic groups with high frequencies of P1 are located in Central Asia and Siberia: 35.4% among Tuvans, 28.3% among Altaian Kizhi,[10] and 35% among Nivkh males.
Modern South Asian populations also feature P1 at low to moderate frequencies.[11] In South Asia it is most frequent among the Muslims of Manipur (33%), but this may be due to a very small sample size (nine individuals). Cases of P1 (M45) reported in South Asia may be unresolved cases or R2 or Q.[11]
| Population group (with ethnolinguistic affiliation) | Paper | N | Percentage | SNPs Tested |
|---|---|---|---|---|
| Tuvinian (Turkic) | Darenko 2005 | 113 | 35.40 | P-M45 |
| Nivkh (isolate) | Lell 2001 | 17 | 35 | P-M45 |
| Altai-Kizhi (Altaians) (Turkic) | Darenko 2005 | 92 | 28.3 | P-M45 |
| Todjin (Turkic) | Darenko 2005 | 36 | 22.2 | P-M45 |
| Chukchi (Chukotkan) | Lell 2001 | 24 | 20.8 | P-M45 |
| Koryak (Chukotkan) | Lell 2001 | 27 | 18.5 | P-M45 |
| Yupik (Eskimo-Aleut) | Lell 2001 | 33 | 18.2 | P-M45 |
| Uighur (Turkic) | Xue 2006 | 70 | 17.1 | P-M45 |
| Kalmyk (Mongolic) | Darenko 2005 | 68 | 11.8 | P-M45 |
| Turkmen (Turkic) | Wells 2001 | 30 | 10 | P-M45 |
| Soyot (Turkic) | Darenko 2005 | 34 | 8.8 | P-M45 |
| Uriankhai (Mongolic) | Katoh 2004 | 60 | 8.3 | P-M45 |
| Khakas (Turkic) | Darenko 2005 | 53 | 7.6 | P-M45 |
| Kazakh (Turkic) | Wells 2001 | 54 | 5.6 | P-M45 |
| Uzbek (Turkic) | Wells 2001 | 366 | 5.5 | P-M45 |
| Khasi-Khmuic (Austro-Asiatic) | Reddy 2009 | 353 | 5.40 | P-M45(xM173) § |
| Mundari (Austro-Asiatic) | Reddy 2009 | 64 | 10.90 | P-M45(xM173) § |
| Nicobarese (Mon-Khmer) | Reddy 2009 | 11 | 0.00 | P-M45(xM173) § |
| Southeast Asia (Austro-Asiatic) | Reddy 2009 | 257 | 1.60 | P-M45(xM173) § |
| Garo (Tibeto-Burman) | Reddy 2009 | 71 | 1.40 | P-M45(xM173) § |
| India (Tibeto-Burman) | Reddy 2009 | 226 | 3.10 | P-M45(xM173) § |
| East Asia (Tibeto-Burman) | Reddy 2009 | 214 | 0.00 | P-M45(xM173) § |
| Eastern India (Indo-European) | Reddy 2009 | 54 | 18.50 | P-M45(xM173) § |
| Iran (Southern Talysh) | Nasidze 2009 | 50 | 4.00 | P-M45(xM124,xM173) |
| Azerbaijan (Northern Talysh) | Nasidze 2009 | 40 | 5.00 | P-M45(xM124,xM173) |
| Mazandarani (Iranian) | Nasidze 2009 | 50 | 4.00 | P-M45(xM124,xM173) |
| Gilaki (Iranian) | Nasidze 2009 | 50 | 0.00 | P-M45(xM124,xM173) |
| Tehran (Iranian) | Nasidze 2004 | 80 | 4.00 | P-M45(xM124,xM173) |
| Isfahan (Iranian) | Nasidze 2004 | 50 | 6.00 | P-M45(xM124,xM173) |
| Bakhtiari (Iranian) | Nasidze 2008 | 53 | 2.00 | P-M45(xM124,xM173) |
| Iranian Arabs (Arabic) | Nasidze 2008 | 47 | 2.00 | P-M45(xM124,xM173) |
| North Iran (Iranian) | Regueiro 2006 | 33 | 9.00 | P-M45(xM124,xM173) |
| South Iran (Iranian) | Regueiro 2006 | 117 | 3.00 | P-M45(xM124,xM173) |
| South Caucacus (Georgian) | Nasidze and Stoneking 2001 | 77 | 3.00 | P-M45(xM124,xM173) |
| South Caucacus (Armenian) | Nasidze and Stoneking 2001 | 100 | 2.00 | P-M45(xM124,xM173) |
| Hvar (Croatian) | Barać et al. 2003 | 14 | ||
| Korčula (Croatian) | Barać et al. 2003 | 6 |
§ These may include members of haplogroup R2.
| Population group | N | P (xQ,xR) | Q | R | Paper | |||
|---|---|---|---|---|---|---|---|---|
| Count | % | Count | % | Count | % | |||
| Gope | 16 | 1 | 6.4 | Sahoo 2006 | ||||
| Oriya Brahmin | 24 | 1 | 4.2 | Sahoo 2006 | ||||
| Mahishya | 17 | 3 | 17.6 | Sahoo 2006 | ||||
| Bhumij | 15 | 2 | 13.3 | Sahoo 2006 | ||||
| Saora | 13 | 3 | 23.1 | Sahoo 2006 | ||||
| Nepali | 7 | 2 | 28.6 | Sahoo 2006 | ||||
| Muslims of Manipur | 9 | 3 | 33.3 | Sahoo 2006 | ||||
| Himachal Pradesh Rajput | 15 | 1 | 6.7 | Sahoo 2006 | ||||
| Lambadi | 18 | 4 | 22.2 | Sahoo 2006 | ||||
| Gujarati Patel | 9 | 2 | 22.2 | Sahoo 2006 | ||||
| Katkari | 19 | 1 | 5.3 | Sahoo 2006 | ||||
| Madia Gond | 14 | 1 | 7.1 | Sahoo 2006 | ||||
| Kamma Chowdary | 15 | 0 | 0 | 1 | 6.7 | 12 | 80 | Sahoo 2006 |
See also
- Ancient population haplogroups are assumed from small ancient sample sizes.
- † Stands for assumed extinction (no living sample of the same haplogroup).
- [2] Entire phylogeny except for haplogroup X, K2b1 clades, K2* clades, and K2c, K2d, as well as P(xM45).
- [12][13][14][15] Ancient DNA samples.
- [16][17][18][19][20][21][22][23][24][25][26][27] Modern populations and ancient Basques.
- [5][28] Y-chromosome DNA haplogroup X.
Notes
Assuming 70,000 years BP for the TMRCA of M168 chromosomes, we estimate the interval of time between the diversification of K-M9 and that of K-P331 to be less than 3,000 years. This rapid diversification has also been assessed using whole Y-chromosome sequence data. In addition, we estimate the total time between the common ancestor of K-M9 and that of P-P295 to be less than 5,000 years, and the time between the common ancestor P-P295 and that of P-P27 to be around 12,300 years.[2]
References
- ↑ Hallast, Pille; Agdzhoyan, Anastasia; Balanovsky, Oleg; Xue, Yali; Tyler-Smith, Chris (2021). "A Southeast Asian origin for present-day non-African human Y chromosomes". Human Genetics. 140 (2): 299–307. doi:10.1007/s00439-020-02204-9. PMC 7864842. PMID 32666166.
- 1 2 3 4 5 6 7 8 9 10 11 12 13 Karafet, Tatiana M.; Mendez, Fernando L.; Sudoyo, Herawati; Lansing, J. Stephen; Hammer, Michael F. (March 2015). "Improved phylogenetic resolution and rapid diversification of Y-chromosome haplogroup K-M526 in Southeast Asia". European Journal of Human Genetics. 23 (3): 369–373. doi:10.1038/ejhg.2014.106. ISSN 1476-5438. PMC 4326703. PMID 24896152.
- ↑ Sanghamitra Sahoo; et al. (2006). "A prehistory of Indian Y chromosomes: evaluating demic diffusion scenarios". Proceedings of the National Academy of Sciences. 103 (4): 843–848. Bibcode:2006PNAS..103..843S. doi:10.1073/pnas.0507714103. PMC 1347984. PMID 16415161.
- ↑ "Downloadable genotypes of present-day and ancient DNA data (compiled from published papers) | David Reich Lab". reich.hms.harvard.edu. David Reich Lab. Archived from the original on 2 November 2019. Retrieved 11 September 2019.
- 1 2 3 "PhyloTree y – Minimal y tree".
- ↑ Basal K2* is now found among indigenous Australian men; the rare K2a* and K2a1 only among living males originating in South Asia and ancient remains from Eastern Europe; and the equally rare K2c, K2d, and K2e only among living males in Southeast Asia.
- ↑ Wells, Spencer (20 November 2007). Deep Ancestry: The Landmark DNA Quest to Decipher Our Distant Past. National Geographic Books. p. 79. ISBN 978-1-4262-0211-7. "Given the widespread distribution of K, it probably arose somewhere in the Middle East or Central Asia, perhaps in the region of Iran or Pakistan."
- ↑ "Downloadable genotypes of present-day and ancient DNA data (compiled from published papers) | David Reich Lab". reich.hms.harvard.edu. David Reich Lab. Archived from the original on 2 November 2019. Retrieved 11 September 2019.
- 1 2 Nagle, N.; Ballantyne, K. N.; Van Oven, M.; Tyler-Smith, C.; Xue, Y.; Taylor, D.; Wilcox, S.; Wilcox, L.; Turkalov, R.; Van Oorschot, R. A.; McAllister, P.; Williams, L.; Kayser, M.; Mitchell, R. J. (2016). "Antiquity and diversity of aboriginal Australian Y-chromosomes". American Journal of Physical Anthropology. 159 (3): 367–381. doi:10.1002/ajpa.22886. PMID 26515539.
- ↑ Derenko, Miroslava; Malyarchuk, Boris; Denisova, Galina A.; Wozniak, Marcin; Dambueva, Irina; Dorzhu, Choduraa; Luzina, Faina; Miścicka-Śliwka, Danuta; Zakharov, Ilia (2006). "Contrasting patterns of Y-chromosome variation in South Siberian populations from Baikal and Altai-Sayan regions". Human Genetics. 118 (5): 591–604. doi:10.1007/s00439-005-0076-y. PMID 16261343. S2CID 23011845.
- 1 2 Sahoo, S. (2006). "A prehistory of Indian Y chromosomes: Evaluating demic diffusion scenarios". Proceedings of the National Academy of Sciences. 103 (4): 843–8. Bibcode:2006PNAS..103..843S. doi:10.1073/pnas.0507714103. PMC 1347984. PMID 16415161.
- ↑ Raghavan, Maanasa; Skoglund, Pontus; Graf, Kelly E.; Metspalu, Mait; Albrechtsen, Anders; Moltke, Ida; Rasmussen, Simon; Stafford Jr, Thomas W.; Orlando, Ludovic; Metspalu, Ene; Karmin, Monika; Tambets, Kristiina; Rootsi, Siiri; Mägi, Reedik; Campos, Paula F.; Balanovska, Elena; Balanovsky, Oleg; Khusnutdinova, Elza; Litvinov, Sergey; Osipova, Ludmila P.; Fedorova, Sardana A.; Voevoda, Mikhail I.; Degiorgio, Michael; Sicheritz-Ponten, Thomas; Brunak, Søren; Demeshchenko, Svetlana; Kivisild, Toomas; Villems, Richard; Nielsen, Rasmus; et al. (2014). "Upper Palaeolithic Siberian genome reveals dual ancestry of Native Americans". Nature. 505 (7481): 87–91. Bibcode:2014Natur.505...87R. doi:10.1038/nature12736. PMC 4105016. PMID 24256729.
- ↑ Rasmussen, Morten; Anzick, Sarah L.; Waters, Michael R.; Skoglund, Pontus; Degiorgio, Michael; Stafford, Thomas W.; Rasmussen, Simon; Moltke, Ida; Albrechtsen, Anders; Doyle, Shane M.; Poznik, G. David; Gudmundsdottir, Valborg; Yadav, Rachita; Malaspinas, Anna-Sapfo; V, Samuel Stockton White; Allentoft, Morten E.; Cornejo, Omar E.; Tambets, Kristiina; Eriksson, Anders; Heintzman, Peter D.; Karmin, Monika; Korneliussen, Thorfinn Sand; Meltzer, David J.; Pierre, Tracey L.; Stenderup, Jesper; Saag, Lauri; Warmuth, Vera M.; Lopes, Margarida C.; Malhi, Ripan S.; et al. (2014). "The genome of a Late Pleistocene human from a Clovis burial site in western Montana". Nature. 506 (7487): 225–229. Bibcode:2014Natur.506..225R. doi:10.1038/nature13025. PMC 4878442. PMID 24522598.
- ↑ Hollard, C.; Keyser, C.; Giscard, P. H.; Tsagaan, T.; Bayarkhuu, N.; Bemmann, J.; Crubézy, E.; Ludes, B. (2014). "Strong genetic admixture in the Altai at the Middle Bronze Age revealed by uniparental and ancestry informative markers". Forensic Science International. Genetics. 12: 199–207. doi:10.1016/j.fsigen.2014.05.012. PMID 25016250.
- ↑ Fregel, Rosa; Gomes, Verónica; Gusmão, Leonor; González, Ana M.; Cabrera, Vicente M.; Amorim, António; Larruga, Jose M. (2009). "Demographic history of Canary Islands male gene-pool: Replacement of native lineages by European" (PDF). BMC Evolutionary Biology. 9 (1): 181. Bibcode:2009BMCEE...9..181F. doi:10.1186/1471-2148-9-181. PMC 2728732. PMID 19650893.
- ↑ Grugni, Viola; Battaglia, Vincenza; Hooshiar Kashani, Baharak; Parolo, Silvia; Al-Zahery, Nadia; Achilli, Alessandro; Olivieri, Anna; Gandini, Francesca; Houshmand, Massoud; Sanati, Mohammad Hossein; Torroni, Antonio; Semino, Ornella (2012). "Ancient Migratory Events in the Middle East: New Clues from the Y-Chromosome Variation of Modern Iranians". PLOS ONE. 7 (7) e41252. Bibcode:2012PLoSO...741252G. doi:10.1371/journal.pone.0041252. PMC 3399854. PMID 22815981.
- ↑ Haber, Marc; Platt, Daniel E.; Ashrafian Bonab, Maziar; Youhanna, Sonia C.; Soria-Hernanz, David F.; Martínez-Cruz, Begoña; Douaihy, Bouchra; Ghassibe-Sabbagh, Michella; Rafatpanah, Hoshang; Ghanbari, Mohsen; Whale, John; Balanovsky, Oleg; Wells, R. Spencer; Comas, David; Tyler-Smith, Chris; Zalloua, Pierre A. (2012). "Afghanistan's Ethnic Groups Share a Y-Chromosomal Heritage Structured by Historical Events". PLOS ONE. 7 (3) e34288. Bibcode:2012PLoSO...734288H. doi:10.1371/journal.pone.0034288. PMC 3314501. PMID 22470552.
- ↑ Bekada, Asmahan; Fregel, Rosa; Cabrera, Vicente M.; Larruga, José M.; Pestano, José; Benhamamouch, Soraya; González, Ana M. (2013). "Introducing the Algerian Mitochondrial DNA and Y-Chromosome Profiles into the North African Landscape". PLOS ONE. 8 (2) e56775. Bibcode:2013PLoSO...856775B. doi:10.1371/journal.pone.0056775. PMC 3576335. PMID 23431392.
- ↑ Rosser, Z. H.; Zerjal, T; Hurles, M. E.; Adojaan, M; Alavantic, D; Amorim, A; Amos, W; Armenteros, M; Arroyo, E; Barbujani, G; Beckman, G; Beckman, L; Bertranpetit, J; Bosch, E; Bradley, D. G.; Brede, G; Cooper, G; Côrte-Real, H. B.; De Knijff, P; Decorte, R; Dubrova, Y. E.; Evgrafov, O; Gilissen, A; Glisic, S; Gölge, M; Hill, E. W.; Jeziorowska, A; Kalaydjieva, L; Kayser, M; et al. (December 2000). "Y-chromosomal diversity in Europe is clinal and influenced primarily by geography, rather than by language". The American Journal of Human Genetics. 67 (6): 1526–43. doi:10.1086/316890. PMC 1287948. PMID 11078479.
- ↑ Pichler, I.; Mueller, J. C.; Stefanov, S. A.; De Grandi, A.; Volpato, C. B.; Pinggera, G. K.; Mayr, A.; Ogriseg, M.; Ploner, F.; Meitinger, T.; Pramstaller, P. P. (2006). "Genetic structure in contemporary south Tyrolean isolated populations revealed by analysis of Y-chromosome, mtDNA, and Alu polymorphisms". Human Biology. 78 (4): 441–464. doi:10.1353/hub.2006.0057. PMID 17278620. S2CID 20205296.
- ↑ Robino, C.; Varacalli, S.; Gino, S.; Chatzikyriakidou, A.; Kouvatsi, A.; Triantaphyllidis, C.; Di Gaetano, C.; Crobu, F.; Matullo, G.; Piazza, A.; Torre, C. (2004). "Y-chromosomal STR haplotypes in a population sample from continental Greece, and the islands of Crete and Chios". Forensic Science International. 145 (1): 61–64. doi:10.1016/j.forsciint.2004.02.026. PMID 15374596.
- ↑ "High Resolution Phylogeographic Map of Y-Chromosomes Reveal the Genetic Signatures of Pleistocene Origin of Indian Populations" (PDF). Archived from the original (PDF) on 26 November 2010.
- ↑ Hirbo, Jibril Boru (2011). "Complex Genetic History of East African Human Populations".
{{cite journal}}: Cite journal requires|journal=(help) - ↑ Sanchez, J.J.; Børsting, C.; Hernandez, A.; Mengel-Jørgensen, J.; Morling, N. (2004). "Y chromosome SNP haplogroups in Danes, Greenlanders and Somalis". International Congress Series. 1261: 347–349. doi:10.1016/S0531-5131(03)01635-2.
- ↑ Cruciani, F; Trombetta, B; Sellitto, D; Massaia, A; Destro-Bisol, G; Watson, E; Beraud Colomb, E; Dugoujon, J. M.; Moral, P; Scozzari, R (July 2010). "Human Y chromosome haplogroup R-V88: a paternal genetic record of early mid Holocene trans-Saharan connections and the spread of Chadic languages". European Journal of Human Genetics. 18 (7): 800–7. doi:10.1038/ejhg.2009.231. PMC 2987365. PMID 20051990.
- ↑ Sascha Willuweit and Lutz Roewer. "YHRD: Y-Chromosome STR Haplotype Reference Database". yhrd.org.
- ↑ Zhong, H.; Shi, H.; Qi, X.-B.; Duan, Z.-Y.; Tan, P.-P.; Jin, L.; Su, B.; Ma, R. Z. (2011). "Extended y Chromosome Investigation Suggests Postglacial Migrations of Modern Humans into East Asia via the Northern Route". Molecular Biology and Evolution. 28 (1): 717–727. doi:10.1093/molbev/msq247. PMID 20837606.
- ↑ "Generation of high-resolution a priori Y-chromosome phylogenies using "next-generation" sequencing data". 13 December 2013. bioRxiv 10.1101/000802.